Showing posts with label DINOSAUR. Show all posts

Tuesday, 17 November 2026

TRACKING DINOSAURS: FOOTPRINTS IN STONE

Dinosaur Track, Tumbler Ridge
Imagine kneeling beside a three-toed depression in a slab of sandstone, your fingers tracing the edges of a print left by a creature that thundered across the Earth over 100 million years ago. 

Dinosaur tracks—known scientifically as ichnites—are time capsules, snapshots of behavior frozen in stone. 

Unlike bones, which tell us what dinosaurs looked like, footprints reveal how they moved, how fast they walked, whether they traveled alone or in herds, and even how they interacted with their environment.

Footprints are classified by shape rather than by exact species, since tracks are trace fossils—evidence of activity, not anatomy. Paleontologists group them into “ichnogenera,” names based on their form.

  • Theropods, the meat-eating dinosaurs like Tyrannosaurus and Allosaurus, left narrow, three-toed prints (tridactyl) with claw marks. Their tracks often show long, slender toes and a V-shaped outline.
  • Ornithopods, the plant-eaters like Iguanodon, also made three-toed prints, but theirs are broader with blunt toes—built for walking on both two and four legs.
  • Sauropods, the long-necked giants, left large round or oval footprints—massive impressions of their column-like feet, often paired with crescent-shaped handprints nearby.
  • Ankylosaurs and stegosaurs left shorter, wider tracks, with toe impressions that resemble stubby, armored stumps.

Theropod Track
You can see spectacular dinosaur tracks across the world and close to home in western Canada. 

The Peace Region of British Columbia boasts the Tumbler Ridge Global Geopark, where hundreds of Cretaceous-era footprints adorn ancient riverbeds. 

In Alberta, the Dinosaur Provincial Park and the Willow Creek tracksites near Lethbridge preserve both sauropod and theropod prints. 

Farther south, classic trackways appear in Utah’s St. George Dinosaur Discovery Site and Colorado’s Picketwire Canyonlands, where sauropods once waded through ancient mudflats.

If you spot a fossil track, look closely at its size, toe count, and depth. 

Is it long and narrow, hinting at a swift predator, or broad and round, evidence of a lumbering herbivore? 

These shapes tell stories—of migration, of pursuit, of entire ecosystems now long vanished—each print a footprint not just in rock, but in time itself.

Definitely take a photo if you are able and if within cell range, drop a GPS pin to mark the spot to share with local experts when you get home.

Sometimes, you can find something amazing but it takes a while for others to believe you. This happened up in Tumbler Ridge when the first dino tracks were found.

Flatbed Creek Dino Tracks
In the summer of 2000, two curious boys exploring a creek bed near Tumbler Ridge, British Columbia, made a discovery that would put their small northern town on the paleontological map. 

While splashing along Flatbed Creek, Mark Turner and Daniel Helm noticed a series of large, three-toed impressions pressed deep into the sandstone—too regular to be random. 

They had stumbled upon the fossilized footprints of dinosaurs that had walked there some 100 million years ago during the Cretaceous. 

Their find sparked scientific interest that led to the establishment of the Tumbler Ridge Museum and later the Tumbler Ridge Global Geopark. 

Since then, paleontologists have uncovered thousands of tracks in the area—from nimble theropods to massive sauropods—etched into the ancient riverbeds and preserving a vivid record of dinosaurs on the move in what was once a lush coastal plain. 


Tuesday, 27 October 2026

SINOSAUROPTERYX AND ARCHAEOPTERYX: FEATHERS, FOSSILS AND THE ORIGINS OF BIRDS

Sinosauropteryx and Archaeopteryx
A feather can change how we see an entire animal.

Preserved beside a delicate skeleton, its faint outline tells us something bones alone cannot: this ancient creature wore plumage. 

Two remarkable fossil animals, Sinosauropteryx and Archaeopteryx, have helped transform our understanding of dinosaurs and the origins of birds.

One was a small predator with a fuzzy coat and a striped tail. The other had feathered wings, sharp teeth and a long, bony tail. 

Together, they invite us to look beyond the familiar image of dinosaurs as entirely scaly giants—and look a little more closely at the birds outside our windows.

SINOSAUROPTERYX: A DINOSAUR IN A FUZZY COAT

Sinosauropteryx lived in what is now northeastern China approximately 125–122 million years ago, during the Early Cretaceous. About a metre long, much of that length taken up by its slender tail, this small theropod walked on two legs and hunted little animals. A fossil preserving a lizard in its stomach offers a wonderfully direct glimpse of dinner.

But the feature that made Sinosauropteryx famous lies around its skeleton.

A fringe of fine, filamentous structures traces parts of the body: the remains of a simple feather covering. These were unlike the broad, neatly vaned flight feathers of a raven or eagle. They would have given the animal a soft, fuzzy appearance.

First discovered in 1996, Sinosauropteryx became a landmark in the study of feathered dinosaurs. Here was evidence that plumage extended beyond early birds into other dinosaur branches.

That distinction matters. A feather covering does not automatically make an animal a flyer.

Research on the preserved colour patterns has also revealed alternating bands along the tail, a darker back, a lighter underside and a dark facial marking described as a “bandit mask.” These patterns suggest camouflage played a role in its life. Countershading—a darker upper surface above a paler belly—can reduce the visual effect of shadows, helping an animal blend into its surroundings.

Even through stone, we can begin to recover something of this little hunter’s appearance.

ARCHAEOPTERYX: AN ANCIENT WING IN LIMESTONE

Travel farther back, to approximately 150 million years ago, and we meet Archaeopteryx.

Its fossils come from the Late Jurassic limestones of southern Germany, particularly the celebrated Solnhofen region. These deposits preserve extraordinary details, including the impressions of feathers surrounding delicate bones.

Look at an Archaeopteryx fossil and the wings immediately catch your eye. Long feathers spread outward from the forelimbs, giving the animal an unmistakably birdlike outline.

Then look again.

There are teeth in the jaws, clawed fingers on the wings and a long tail supported by a series of vertebrae. This combination of features makes Archaeopteryx especially valuable for understanding the early evolution of birds.

Its name means “ancient wing”—a fitting name for an animal that has prompted generations of palaeontologists to ask how dinosaurs took to the air.

Could it fly? Research examining the internal geometry of its wing bones supports active, flapping flight. Its capabilities and wing stroke, however, differed from those of modern birds. The evidence points towards short flights rather than the sustained aerial journeys we see in many birds today.

FEATHERS BEFORE FLIGHT

There is a delightful wrinkle in this story: the fuzzy, flightless Sinosauropteryx lived millions of years after the winged Archaeopteryx.

They do not form a simple sequence in which one became the other. Evolution branches. Different dinosaur lineages lived with different combinations of feathers, skeletons and ways of moving.

The broader fossil record shows that feathers were present in dinosaurs that could not fly. Early plumage may have helped with insulation, display and other functions before feathers became part of the equipment for aerial travel. The flight feathers of birds belong within that longer evolutionary history.

Birds are living theropod dinosaurs. The chickadee investigating a branch, the gull turning above the shoreline and the raven watching you with considerable interest all belong to a dinosaur lineage that survives today.

FOLLOWING THE STORY IN OSLO

If your travels take you to Norway, the Natural History Museum in Oslo, or Naturhistorisk museum, offers an opportunity to explore this connection between dinosaurs and birds.

The museum has featured Sinosauropteryx and Archaeopteryx through reconstructed displays, bringing their feathered forms into three dimensions. Its exhibition material describes a downy Sinosauropteryx model, while reporting on its bird evolution displays documents a fully feathered Archaeopteryx reconstruction. These are representations of the ancient animals; visitors should check individual labels to distinguish models, casts and original fossils.

The museum’s current permanent exhibition, Evolution of Life, is housed in Brøggers hus. It follows life through geological time, exploring changing ecosystems and important evolutionary developments among animals and plants. Fossils provide the clues connecting these ancient worlds.

Located at Sars’ gate 1, 0562 Oslo, Norway, the museum grounds include the Botanical Garden. Beyond palaeontology, visitors can explore exhibitions on animals, minerals, geology and climate. Tøyen metro station is approximately a six-minute walk from the southern entrance in Monrads gate. Check the museum’s official website for current exhibitions, opening hours and admission information, particularly if you hope to see a specific display.

Lead Image: Asset ID: 2704872271

Tuesday, 13 October 2026

NORELLRAPTOR: A FEATHERED DINOSAUR AND THE MANY PATHS TO FLIGHT

Norellraptor barsboldi
We are accustomed to imagining the Mesozoic through its giants: enormous herbivores shaking the ground and predators with teeth the size of bananas. 

Yet some of the most revealing discoveries arrive on a much smaller scale.

While I imagine it would go horribly wrong, I still cannot get over the charm of this cutie and the wonderfully disarming notion of a dinosaur small enough to hold in your arms.

Meet Norellraptor barsboldi, a newly described feathered dinosaur from northeastern China.

Its remarkably complete skeleton measures just 57 centimetres long—roughly the length of a small Common Raven, though with very different proportions—and parts of its plumage remain preserved alongside the bones.

Here is an animal whose delicate remains give us a peek at one of evolution’s most extraordinary achievements: flight.

Published in Nature Communications on 29 September 2026, the new research adds another branch to a story that grows more interesting with every feathered fossil.

The question is how different dinosaur lineages assembled the anatomical features associated with taking to the air.

Norellraptor belonged to the microraptorines, small predatory dinosaurs closely related to birds. 

Its fossil comes from the Lower Cretaceous Jiufotang Formation in Liaoning, China—a province celebrated for its jade carvings, which also holds extraordinary treasures in its fossil beds.

Members of this group are famous for an unusual arrangement: some carried long feathers on both their arms and legs, creating the possibility of several aerodynamic surfaces.

Try imagining that silhouette. A small dinosaur with feathered limbs and a long tail looks very different from the familiar outline of a sparrow. It invites an artist’s curiosity, but also a scientist’s questions.

How were those limbs positioned? What could the feathers do? How much can a flattened fossil tell us about an animal moving through three-dimensional space?

Those questions make the distinction between evidence and reconstruction especially valuable. Preserved feathers give us something tangible to study. Reconstructing how the whole animal moved requires further interpretation.

The research team examined both the skeleton and the microscopic structure of a forelimb bone. They tell us that this individual was at least three years old when it died. But how did they know? An excellent question. Fossils can preserve more than an outline; the tissues inside its bones can also hold clues to its growth.

The larger finding emerged when the team compared evolutionary changes in microraptorines with those in the bird lineage. 

Around 30 per cent of the anatomical features identified as evolutionary innovations in microraptorines also appeared independently along the bird branch. Crucially, the shared features emerged in different sequences.

Imagine finding two complicated machines with several similar components. Their resemblance alone cannot tell you whether they were assembled through the same process. You would also want to know when each component appeared and how it worked with the parts already present.

The study supports the interpretation that different evolutionary pressures helped shape flight-related adaptations in these closely related groups. Similarities between them need not all represent a single inherited package of aerial abilities.

It is an enticing result, though further fossils and evidence of bone growth will be needed to test how widely this pattern applies. Norellraptor contributes to the discussion rather than closing it.

That is part of what I love about palaeontology. Each discovery gives us another opportunity to replace a tidy picture with a richer one. Evolution has no obligation to follow the clean sequence we might choose for a museum wall. Its history is branching, and fossils allow us to examine those branches one extraordinary specimen at a time.

Personally, while I am excited by the fossil bones they found, it is the feathers that steal my heart. It will be very exciting to see what we learn from them.

A feathered fossil in stone and a bird outside the window belong to the same unfolding conversation. One helps us ask how aerial adaptations arose. The other lets us watch what one surviving branch can do.

There is a lovely way to carry this story into the present. Watch a crow settle onto a branch, a gull adjust its wings above the shoreline, or a small songbird disappear into the trees. Living birds are dinosaurs, carrying that deep evolutionary history into our everyday world.

Each makes the larger story wonderfully immediate.

Sunday, 4 October 2026

TRICERATOPS: THE HERD THAT CHANGED THE STORY

Triceratops, Leiden, Netherlands
At the Naturalis Biodiversity Center in Leiden, the Netherlands, a visit to the dinosaur gallery is also a glimpse into the work of a research institute. 

Naturalis studies life on Earth through its vast natural history collection, and its dinosaur discoveries have given us something remarkable to talk about.

Naturalis Biodiversity Center in Leiden traces its beginnings to 1820, when King William I founded the Netherlands’ National Museum of Natural History by bringing together existing collections and scientific cabinets. 

Its holdings grew through research expeditions, collections from other Dutch institutions and gifts from private collectors. That history has a difficult side: some specimens were collected in colonial settings under circumstances Naturalis now investigates through provenance research. 

Today, the collection holds more than 43 million objects, though only a fraction are on display. Visitors can meet Trix the T. rex and Triceratops in the Dinosaur Age gallery, explore mammoth fossils and other Ice Age animals, and discover how life has changed over billions of years.

It is there wonderful triceratops display you see in the photo here. It showcases Triceratops horridus: three horns, a broad bony frill, a sturdy plant eater’s body, and a face that has been a dinosaur icon for generations. 

It lived in North America near the end of the Cretaceous, roughly 67 million years ago.

These fellows are some of my favourite dinosaurs. I had a lovely figurine of one that I played with as a youth and still sits on my shelf to this day.

We often picture Triceratops roaming in herds, but fossils had offered little firm evidence for that familiar scene. Then Naturalis researchers uncovered the remains of five individuals together in Wyoming. Naturalis excavated six Triceratops in Wyoming overall, but five were found together in the bonebed that became the museum’s herd.

The five Triceratops were found by a Naturalis Biodiversity Center expedition team on a ranch near Newcastle, Wyoming, in 2013. The team was searching for Tyrannosaurus fossils when it encountered Triceratops bones. Further excavation revealed remains of at least five individuals together; the work continued over several years under research leader Anne Schulp. 

Anne Schulp is a vertebrate palaeontologist at Naturalis and a professor at Utrecht University. Trained in Earth Sciences, with a doctorate focused on mosasaurs, Schulp studies dinosaurs, ancient marine reptiles and fossil footprints, and continues to lead the research group investigating Naturalis’s Triceratops herd.

Years of excavation and study led them to conclude that these animals lived and died as a group. In 2024, Naturalis brought all five together for the first public display of this extraordinary herd.

That is the thrill of palaeontology: even the dinosaurs we think we know can surprise us. One fossil tells us about an animal. Five found together may tell us something about how they lived.

The herd’s Leiden exhibition ended in August 2025, and the fossils are now travelling internationally. This photo captures a special chapter in their story.

Image ID: 2559349211

Thursday, 1 October 2026

ANKYLOSAURUS: THE DINOSAUR WITH BUILT-IN SECURITY

Ankylosaurus
Ankylosaurus took “don’t mess with me” to a whole new level: body armour, a giant tail club, and absolutely no interest in becoming someone else’s lunch.

This heavily armoured dinosaur lived in North America near the end of the Cretaceous. 

Bony plates protected its broad back, while a low-slung body kept its softer belly close to the ground. It spent its days eating vegetation and, presumably, being an absolute nuisance to anything hoping for an easy lunch.

Then there was the tail. The “handle” was made of stiffened, interlocking bones, with a hefty bony knob at the end. 

Ankylosaur tail clubs could deliver a powerful sideways blow. Bam! Was that club used against predators, rival ankylosaurs, or both? 

Fossils from another club-tailed ankylosaur, Zuul, show injuries consistent with blows from other tail clubs. That gives us a fascinating clue, though it doesn’t tell us every way Ankylosaurus used its own.

My favourite thing about Ankylosaurus is the contrast: a plant eater dressed for battle. No sharp teeth, no dramatic chase scene—just armour, a formidable tail, and a strong suggestion to give it some personal space.

Sunday, 27 September 2026

DEINONYCHUS: THE REAL DINOSAUR BEHIND JURASSIC PARK'S RAPTORS

Deinonychus antirrhopus
If you met Deinonychus in the Early Cretaceous, your first thought might be, “What a splendid bird.” 

Your second thought, if you were a small animal, would probably be, “Oh dear.”

Deinonychus antirrhopus was a two-legged, meat-eating dinosaur that lived in what is now North America roughly 115 to 108 million years ago. 

Its name means “terrible claw”, which is charmingly direct for palaeontology. There is no need to work through three layers of Latin to discover that this animal had a rather alarming feature attached to each foot.

On the second toe of each hind foot sat a large, curved claw. Deinonychus could hold that toe off the ground as it moved, keeping the claw ready for action. 

It also had sharp teeth and a long, stiffened tail that helped it balance. Imagine a feathered predator built for agility, with excellent equipment and absolutely no interest in your personal space.

Deinonychus skull
In the 1960s, palaeontologist John Ostrom found Deinonychus fossils in Montana. 

When he described the animal in 1969, its light build and active-looking anatomy challenged the popular image of dinosaurs as slow, lumbering creatures. 

Deinonychus helped set off the “dinosaur renaissance”: a fresh look at how dinosaurs moved, behaved and, eventually, how closely some were related to birds.

That makes it a scientific celebrity, even if Hollywood gave most of its screen time to someone else. 

The famous “Velociraptors” of Jurassic Park drew heavily on Deinonychus. Actual Velociraptor was smaller. Deinonychus, meanwhile, has spent decades watching another dinosaur accept the applause. 

Fossils of Deinonychus have been found alongside the plant-eating dinosaur Tenontosaurus. Researchers have also identified marks on Tenontosaurus bones that they interpret as Deinonychus bites. It seems clear that Tenontosaurus could end up as food. 

Whether Deinonychus hunted it alone, hunted in groups, scavenged it, or did some combination of these remains harder to pin down.

That is the joy and occasional frustration of palaeontology: a fossil can tell us who came to dinner without providing the seating chart.

We also do not have direct fossil feathers from Deinonychus itself. Its close relatives and its place on the dinosaur family tree make a feathered appearance a strong scientific interpretation, though. The scaly movie raptor may have had good lighting, but a fluffy Deinonychus is much closer to how many picture the real animal.

So give Deinonychus its due. It was a formidable Cretaceous predator, a surprise star of dinosaur science and quite possibly the owner of the most consequential toenail in palaeontology. Cute, deadly and a lovely fossil to behold!

Thursday, 17 September 2026

WHEN DIPLODOCUS CROSSED THE ATLANTIC

Palaeontologists have just identified the first confirmed Diplodocus fossils found outside North America. 

Until this discovery, confirmed Diplodocus fossils were known only from the Morrison Formation of the western United States.

The remains—14 tail vertebrae and several chevron bones—were recovered near El Castellar in Teruel, Spain. 

They belonged to an animal roughly 25 metres long that lived about 150 million years ago.

This is a terrific story because the fossils do more than place a familiar dinosaur somewhere new. They suggest that dinosaurs travelled between North America and Europe while the young Atlantic Ocean was opening, possibly crossing temporary land bridges during periods of lower sea level. 

For more than a century, Diplodocus appeared to be a thoroughly North American dinosaur. 

Its fossils were known from the Late Jurassic Morrison Formation of the western United States, where these wonderfully long-necked herbivores wandered across ancient floodplains alongside Stegosaurus, Allosaurus and other familiar Jurassic giants.

Now, Diplodocus has turned up somewhere entirely unexpected: Spain.

Palaeontologists from the Fundación Dinópolis identified 14 exceptionally well-preserved tail vertebrae and several chevron bones from the La Tejería fossil site near El Castellar in Teruel. The bones are about 150 million years old and represent the first confirmed Diplodocus discovered outside North America.

The Spanish animal was no dainty traveller. Researchers estimate that it reached approximately 25 metres in length—about the length of two city buses parked end to end. Most of that impressive silhouette consisted of an extraordinarily long neck and an even longer, whip-like tail, balanced around a comparatively compact body and remarkably small head.

The fossil was identified through distinctive features in its tail bones. These included elongated vertebral centra, large air-filled cavities within the vertebrae, deep grooves along their undersides and forked chevrons. 

Chevrons are bones attached beneath the tail vertebrae that helped protect blood vessels while providing anchoring points for muscles. Together, these anatomical clues placed the Spanish specimen firmly within the genus Diplodocus and close to the North American species Diplodocus hallorum.

Its presence in Spain raises a delicious prehistoric question: how did a dinosaur associated with the American West reach Jurassic Europe?

It did not swim across the modern Atlantic—and frankly, a 25-metre sauropod doing the dog paddle would have been memorable. During the Late Jurassic, the Atlantic Ocean was only beginning to open as the supercontinent Pangaea broke apart. 

North America and Europe were much closer together, and changes in sea level may occasionally have exposed islands or temporary land connections. These routes could have allowed dinosaurs to move between the continents in stages.

The discovery supports growing evidence of faunal exchange between North America and the Iberian Peninsula. 

Dinosaurs with close North American connections, including stegosaurs and large theropods, have also been discovered in Portugal and Spain. Iberia may have acted as an important gateway between ancient continents while the young Atlantic widened around it.

The new specimen also adds to the remarkable collection of giant sauropods known from Teruel. These included Turiasaurus, a massive European sauropod belonging to a very different evolutionary branch, and Losillasaurus, another enormous long-necked herbivore. 

Late Jurassic Spain was evidently not short of giants—or of the vegetation required to keep them fed.

This discovery does not yet tell us whether the Spanish animal belonged to a known species of Diplodocus or represents one that is new to science. More fossils will be needed before researchers can answer that question. The bones nevertheless demonstrate something extraordinary: Diplodocus was not confined to North America after all.

Its enormous feet once touched European soil, and its tail stretched across more than a landscape. It reached across our assumptions about how Jurassic dinosaurs travelled, dispersed and responded to a planet whose continents were slowly becoming worlds apart.

The research was published in the Journal of Vertebrate Paleontology on September 15, 2026. 

The original fossils are now displayed at the Museo Aragonés de Paleontología in Dinópolis, Teruel. 

If you're planning a visit, Teruel is about:

  • 145 km northwest of Valencia
  • 180 km south of Zaragoza
  • 300 km east of Madrid

Valencia is the nearest major international city and the most convenient reference point for travelers. It is off the beaten track but worth the trip.

The research was published on September 15, 2026, making it wonderfully fresh. It gives us giant dinosaurs, continental drift, prehistoric migration and a splendid tail—all excellent ingredients for a tasty read.

Here's the paper for your enjoyment: https://www.eurekalert.org/news-releases/1143855?utm_source=chatgpt.com


Tuesday, 8 September 2026

SUE THE T. REX: THE QUEEN—OR KING—OF CHICAGO

SUE, the T Rex at the Field Museum, Chicago
Standing more than 12 metres (40 feet) long and roughly 4 metres (13 feet) tall at the hips, SUE is one of the largest, most complete and best-preserved specimens of Tyrannosaurus rex ever discovered. 

Their fossilized bones are displayed in a private gallery within the Griffin Halls of Evolving Planet at Chicago’s Field Museum—and yes, SUE has their own suite. After 67 million years, it seems only fair.

Despite the familiar name, scientists do not know whether SUE was biologically female or male. I think of SUE as going with the pronouns they/them. 

The dinosaur is named for fossil hunter and explorer Sue Hendrickson, who discovered several enormous vertebrae protruding from an eroding bluff near Faith, South Dakota, on August 12, 1990. 

Hendrickson was working with the Black Hills Institute of Geological Research when a flat tire gave her time to explore a nearby outcrop. It was possibly the most productive flat tire in palaeontological history. Six people spent 17 days excavating the skeleton.

Field Museum of Natural History, Chicago, USA
After a lengthy ownership dispute, the Field Museum purchased SUE at auction in 1997. The bones arrived in Chicago still partly enclosed in the surrounding rock, or matrix. 

Preparing them was no small undertaking: twelve skilled fossil preparators spent approximately 30,000 hours removing rock, cleaning, repairing and stabilizing the fossils. 

The work was carried out in preparation laboratories at the Field Museum and Disney’s Animal Kingdom, where visitors could watch the painstaking process through glass.

The preparation team included Field Museum fossil specialists Bill Simpson and Paul Brinkman, along with other museum preparators and volunteers. 

Far from simply brushing away a little dust, they used fine hand tools, air scribes, adhesives and an extraordinary amount of patience to free each bone without damaging its surface. Altogether, the preparation required the equivalent of about twelve person-years of work. 

Another 20,000 hours went into studying, casting, mounting and constructing the original exhibition. It was a true labour of love.

About 250 of the estimated 380 bones in a T. rex skeleton are represented, making SUE about 90 percent complete by bone volume. The mounted skeleton contains mostly genuine fossil bone, while specially coloured replicas fill some gaps. 

SUE’s immense original skull—too heavy and scientifically valuable to place safely on the neck—is exhibited separately at eye level. A lighter cast sits on the mounted skeleton that you see in the photo here.

SUE provides an unusually complete look at the anatomy of an adult Tyrannosaurus rex. Detailed study and CT scanning of the skeleton and skull have helped researchers examine the construction of the jaws, braincase, vertebral column, limbs and sensory systems. 

SUE also preserves a furcula, or wishbone, adding to the extensive anatomical evidence linking theropod dinosaurs with birds. The beautifully preserved gastralia—rib-like bones positioned beneath the ordinary ribs—show that T. rex possessed a deep, muscular belly rather than the fashionably shrink-wrapped waist once given to dinosaurs in older reconstructions. These bones may also have helped move air through the respiratory system.

SUE represents the highly specialized endpoint of a much longer tyrannosaur evolutionary story. The earliest tyrannosauroids were relatively small, lightly built hunters. 

Over tens of millions of years, members of the group developed increasingly powerful senses, reinforced skulls, deep jaws and bone-crushing bites. Fossils such as the horse-sized Timurlengia euotica, which lived about 90 million years ago, indicate that sophisticated brains and sharp sensory abilities evolved before tyrannosaurs became gigantic. 

Later tyrannosaurids shifted much of the business of catching and processing prey to the head, while the forelimbs became shorter and the body grew truly colossal.

SUE shows us the result of that transformation: a huge, powerfully balanced predator with a massive skull, robust hind limbs and a long tail acting as a counterweight. This was not simply an oversized version of an earlier meat-eating dinosaur. 

Tyrannosaurus rex was an evolutionary specialist, built around an exceptionally strong bite, keen senses and the ability to dominate the final Late Cretaceous ecosystems of western North America.

The skeleton also preserves the history of one remarkably battered life. SUE suffered injuries and disease, including healed ribs, damaged vertebrae, arthritis and holes in the lower jaw associated with infection. 

Bone growth records indicate that SUE experienced a dramatic adolescent growth spurt, reached adult size at approximately 19 years of age and lived to around 28—an elderly individual by known T. rex standards. 

At one point during the teenage years, SUE may have gained roughly two kilograms, or 4.5 pounds, every day. That is what happens when adolescence involves fewer awkward school photographs and considerably more meat.

One skeleton cannot explain the entire evolution of Tyrannosaurus rex, but SUE provides an essential anatomical benchmark against which less complete specimens can be compared. Their nearly complete body helps palaeontologists distinguish evolutionary features shared by the species from injuries, individual variation and changes produced during growth.

SUE is therefore much more than an impressive museum mount. This extraordinary fossil records the evolutionary culmination of the tyrannosaur lineage, the rapid growth of a gigantic predator and the bruising reality of life near the end of the Age of Dinosaurs.

And after surviving infections, injuries, 67 million years underground and 30,000 hours of fossil preparation, SUE still looks remarkably pleased with themselves.

Lead Image: Asset ID: 2569246875. SUE at the Field Museum of Natural History, Chicago, Illinois, USA

Friday, 28 August 2026

TINY DINOSAUR WITH BIG SECRETS: ALNASHETRI

Alnashetri cerropoliciensis
Slip back 90 million years and wander the sun-baked floodplains of Patagonia, where the giants get all the glory—but it’s the tiny, fleet-footed oddballs that hold the real secrets.

Meet Alnashetri cerropoliciensis, a delicate little dinosaur with a big story to tell. We’re talking under two pounds soaking wet—lighter than your average house cat—but armed with clues powerful enough to untangle one of palaeontology’s most puzzling lineages: the alvarezsaurs.

These were no ordinary theropods. Picture a bird-like body, teeth reduced to tiny pegs, and arms so short they seem almost comical—until you notice the business end: a single, oversized claw built for digging. Think ant-eater, but make it a dinosaur.

For decades, alvarezsaurs have been a bit of a head-scratcher. Beautiful fossils from Asia told part of the tale, but their South American cousins? Fragmentary, elusive, maddeningly incomplete. Then along comes Alnashetri—a near-complete skeleton pulled from the fossil-rich beds of La Buitrera—and suddenly the story sharpens into focus.

And what a twist it is.

This wee creature shows us that alvarezsaurs didn’t shrink because they specialized—they were already pint-sized before evolving their quirky, ant-snuffling toolkit. Longer arms, bigger teeth—Alnashetri still carries the echoes of its less specialized ancestors. It’s evolution mid-sentence, frozen in bone.

Even better, it’s fully grown. No baby here. Just a tiny adult navigating a world of much larger predators with speed, stealth, and a very particular taste in snacks.

The real magic? This fossil acts like a Rosetta Stone for the group, giving scientists a reference point to decode those scrappy, half-told specimens tucked away in collections around the world. Suddenly, the family tree starts to make sense.

And the plot thickens.

Rather than evolving in one place and spreading outward, these curious little dinosaurs likely trace their roots back to Pangaea—before the continents tore themselves apart. As the landmasses drifted, so too did their descendants, leaving behind a scattered but connected fossil trail across the globe.

So here we have it: a tiny dinosaur rewriting a very big story. A cheeky wee dino challenging what we thought we knew!

Reference: https://www.nature.com/articles/s41586-026-10194-3

Thursday, 27 August 2026

DINOSAUR RIVALRY: MANTELLISAURUS

Mantellisaurus atherfieldensis 
This story begins some 125 million years ago on the lush floodplains of what is now the Isle of Wight, back in the Cretaceous.

Forget the cool, windswept English coastline of today. This was a warm, subtropical world of broad rivers, oxbow lakes and sprawling wetlands, where towering conifers, cycads and tree ferns sheltered one of Europe's richest dinosaur ecosystems. 

Early flowering plants were just beginning to appear, while insects buzzed through the forests and reptiles called across the floodplains.

Here, herds of Mantellisaurus atherfieldensis browsed on tender vegetation. At seven to eight metres (23–26 feet) long, these elegant herbivores were among the largest animals in their world. 

Their long hind limbs suggest they could move surprisingly quickly when needed—particularly if a hungry Neovenator emerged from the trees. 

Nothing encourages cardio quite like becoming someone else's lunch.

Its hands were every bit as remarkable as the rest of the animal. Projecting from each was a formidable thumb spike. Victorian artists loved depicting these dinosaurs charging into battle like armoured knights, but the reality was likely less theatrical. 

The spikes probably served as defensive weapons, may have helped settle disputes during the breeding season and perhaps even assisted in pulling down stubborn vegetation. Evolution has always appreciated a multitool.

The elongated fifth finger tells another story. Unlike the stout thumb, it was surprisingly flexible, capable of curling around branches to draw foliage closer—a wonderfully delicate adaptation for an animal weighing well over a tonne.

This specimen was discovered in 1914 by geologist Reginald Walter Hooley in the Upper Vectis Formation near Atherfield on the Isle of Wight. 

Described in 1917 and formally named Iguanodon atherfieldensis in 1925, it spent more than eighty years as a member of the ever-growing Iguanodon family.

That changed in 2007, when American palaeoartist and researcher Gregory S. Paul recognised that it was something quite different. 

More lightly built, with longer limbs and closer evolutionary ties to the African iguanodontian Ouranosaurus, it deserved a genus of its own. Paul named it Mantellisaurus, honouring Dr Gideon Algernon Mantell, the Sussex physician whose discoveries helped launch the science of dinosaurs.

Mantell's story is one of brilliance, perseverance and one of Victorian science's greatest rivalries.

In 1822, he described Iguanodon, only the second dinosaur ever scientifically named.

Mantell spent decades collecting fossils and championing these extraordinary animals, only to find himself increasingly at odds with the formidable anatomist Sir Richard Owen.

Owen coined the word Dinosauria and later became the driving force behind London's Natural History Museum, but he also had a habit of eclipsing rivals—and few felt that more keenly than Mantell. The two men disagreed about almost everything, from dinosaur anatomy to broader questions of evolution, as they emerged in Victorian science.

Mantell increasingly recognised that these animals were active, lightly built and far more dynamic than giant lizards. Owen preferred to reconstruct them as slow, heavily built, rhinoceros-like reptiles that fit comfortably within his creationist view of nature.

When Benjamin Waterhouse Hawkins created the famous Crystal Palace dinosaurs during the 1850s, it was Owen's interpretation that guided the sculptures. 

Visitors marvelled at enormous reptilian beasts, including an Iguanodon sporting what appeared to be a horn proudly perched upon its nose.

As science advanced—and as more complete skeletons were discovered, particularly the spectacular Bernissart specimens from Belgium—we learned that the famous "horn" was, in fact, the thumb spike.

One of the most iconic mistakes in palaeontology had become one of its best-known corrections.

Thursday, 20 August 2026

PROBAINOGNATHUS: FROM BITE TO SOUND

Among the towering dinosaurs, enormous marine reptiles and other spectacular fossils at the Natural History Museum Abu Dhabi is a much smaller creature that tells one of evolution’s most extraordinary stories.

It is a fossil of Probainognathus, a small, predatory cynodont from the Triassic Period of Argentina. At first glance, it is not especially imposing. 

It lacks the theatrical horns of Triceratops, the banquet-sized teeth of Tyrannosaurus rex and the general architectural confidence of a sauropod.

But look closely at its skull—particularly its jaw—and you are staring at a chapter in the evolutionary history of every mammal alive today.

That includes whales, bats, elephants, shrews, platypuses, cats, dogs and the primate currently reading this article.

Tiny creature. Enormous family consequences.

BEFORE THERE WERE MAMMALS

To understand Probainognathus, we need to travel back roughly 235 million years to the early part of the Late Triassic Period.

The world looked nothing like it does today. The continents were assembled into the supercontinent Pangaea. Dinosaurs had only recently appeared and had not yet become the dominant large animals of terrestrial ecosystems. 

Crocodile-line archosaurs, early dinosaur relatives, large amphibians and a wonderful assortment of synapsids occupied the land.

Synapsids are the great evolutionary lineage to which mammals belong. They diverged from the lineage leading to reptiles more than 300 million years ago. Although older books often describe many early synapsids as “mammal-like reptiles,” this is misleading. They were not reptiles slowly deciding to become mammals. Synapsids and reptiles were separate branches of the amniote family tree.

One branch eventually produced dinosaurs and birds. Another produced us.

Within the synapsids arose the therapsids, and within the therapsids evolved the cynodonts. The name Cynodontia means “dog teeth,” although most cynodonts would not have looked particularly dog-like. The name refers to features of their teeth and jaws rather than any secret Triassic ambition to become golden retrievers.

Cynodonts included animals ranging from sturdy plant-eaters to quick little predators. Over millions of years, members of this group developed many features associated with mammals: differentiated teeth, enlarged jaw muscles, changes in the palate, more efficient breathing, increasingly upright limbs and a lower jaw dominated by a single large bone called the dentary.

The evolutionary story did not unfold as a straight march from primitive to advanced. It was a branching, experimental process involving many species, most of which left no living descendants. Probainognathus belongs to one of the branches close to the part of the cynodont tree from which mammals eventually emerged.

It was not quite a mammal. It was certainly not our direct, neatly labelled great-great-grandparent. It was a non-mammalian cynodont whose anatomy preserves a revealing combination of older and more mammal-like features.

Evolution, as usual, was tinkering.

HONEY, I MADE A NEW FRIEND: MEET PROBAINOGNATHUS

The best-known species, Probainognathus jenseni, was formally named by American palaeontologist Alfred Sherwood Romer in 1970. Its fossils were collected from the Chañares Formation in La Rioja Province, northwestern Argentina.

The name Probainognathus is generally translated as “progressive jaw,” a direct reference to the feature that made the animal scientifically important. 

The species name honours fossil collector James A. Jensen, who led the team associated with the discovery of the original material.

Radiometric dating of volcanic minerals has placed the principal fossil-bearing interval of the Chañares Formation at approximately 236 to 234 million years old. The formation had previously been regarded as Middle Triassic, but more precise dating showed that much of its famous vertebrate assemblage belongs near the beginning of the Late Triassic.

At that time, what is now northwestern Argentina lay within a volcanically active rift basin. Rivers, lakes and floodplains supported an ecosystem filled with dicynodonts, cynodonts, early archosaur relatives and some of the animals living close to the origin of dinosaurs.

Volcanic ash and sediment repeatedly entered the landscape. In some areas, animals were buried within concretions—hard masses of mineral-rich rock that formed around their remains. These deposits preserved a remarkable record of Triassic terrestrial life, including animals that would otherwise have been very easy to overlook.

Probainognathus was small, lightly built and probably no more than about half a metre long, although complete skeletons are rare and estimates vary. Its skull was only several centimetres in length. It likely moved on four legs and probably hunted insects and other small animals, perhaps taking tiny vertebrates when the opportunity arose.

In other words, it was living through one of the most dramatic periods in vertebrate evolution while pursuing the equally urgent matter of finding something crunchy for dinner.

TEETH MADE FOR BUSINESS

The jaws of Probainognathus held differentiated teeth rather than a uniform row of nearly identical pegs.

At the front were small incisors. Behind them were enlarged canine teeth, followed by postcanine teeth adapted for processing food. Some specimens show serrations on the canines, suggesting that these teeth were useful for gripping and cutting flesh.

This regional specialization of the teeth—incisors for nipping, canines for piercing and postcanines for slicing or crushing—was an important development in cynodont evolution. Mammals would take this dental division of labour to remarkable extremes.

Think of the front teeth of a beaver, the canines of a wolf and the grinding molars of a horse. Each part of the tooth row performs a different job. Probainognathus did not possess the sophisticated chewing system of a modern mammal, but its teeth were already part of that broader evolutionary experiment.

Its skull also provided space for substantial jaw muscles. Changes in the skull and lower jaw allowed cynodonts to bite more effectively and process food more efficiently. That may have helped support higher levels of activity and, in later mammalian relatives, the energetic demands associated with endothermy.

Whether Probainognathus itself had fur or maintained a fully mammal-like body temperature cannot be established directly from its bones. Some cynodont relatives probably possessed whiskers or hair-like coverings, but soft tissues are rarely preserved. 

It is tempting to reconstruct Probainognathus as a fuzzy, bright-eyed little creature. That may be reasonable, but we should acknowledge where fossil evidence ends, and our fondness for adding whiskers begins.

THE JAW THAT CHANGED EVERYTHING

The real evolutionary celebrity in this fossil is the jaw joint.

Most non-mammalian jawed vertebrates use two small bones to connect the lower jaw to the skull. The quadrate bone in the skull meets the articular bone at the back of the lower jaw.

Living mammals do things differently. Our lower jaw consists almost entirely of one bone, the dentary, which articulates directly with the squamosal region of the skull. The old quadrate and articular bones no longer serve as the main jaw hinge.

They are now inside our ears.

Over the course of synapsid evolution, the quadrate became the incus, or anvil, while the articular became the malleus, or hammer. Together with the stapes, they form the three tiny middle-ear bones that transmit sound vibrations toward the inner ear.

Pause for a moment to admire the audacity of this arrangement. Bones that once helped an ancestor bite eventually became bones that help us hear.

No engineering committee proposed this reassignment. Evolution modified existing structures over many generations, gradually changing their size, position and function.

For this transition to occur, however, the lower jaw required a new way to attach securely to the skull. 

Several groups of advanced cynodonts developed additional contact between bones around the jaw joint while retaining the older quadrate–articular connection. For a time, these animals effectively possessed a transitional arrangement involving both the ancestral jaw hinge and a new secondary contact.

When Romer described Probainognathus, he interpreted its anatomy as showing an incipient articulation between the dentary and squamosal—the bones that form the mammalian jaw joint. This interpretation inspired the name “progressive jaw.”

Later studies have complicated that tidy picture. Some researchers concluded that the additional contact may have involved the surangular, one of the smaller bones behind the dentary, rather than a fully developed dentary–squamosal joint. 

More recent research has also shown that mammal-like jaw contacts arose independently in more than one cynodont lineage.

The route to the mammalian jaw was not a single anatomical escalator travelling smoothly upward. It was more like several teams attempting renovations at once, occasionally arriving at similar solutions.

Even with those scientific revisions, Probainognathus remains valuable. Its reduced postdentary bones, enlarged dentary and changing relationships among the bones at the back of the skull capture an important stage in the broader transformation of the cynodont jaw and ear.

It reminds us that transitional fossils are not required to be perfectly halfway between two modern categories. They document populations in which anatomical systems were being reorganized, often in complicated and unexpected combinations.

WHY BECOME SMALL?

Many of the cynodonts nearest the origin of mammals were small animals. Miniaturization may have played a major role in reshaping their skulls.

A smaller animal experiences different mechanical pressures. Its jaw bones become more delicate, its food may require precise processing, and hearing higher-frequency sounds can become increasingly useful. Small nocturnal or crepuscular hunters able to detect insects rustling through vegetation would have benefited from improved hearing.

At the same time, the dentary was becoming larger and stronger while the other bones of the lower jaw were shrinking. Once the new jaw articulation could bear the forces of biting, the old joint bones were increasingly free to specialize in transmitting sound.

The transition did not happen in one species or during one convenient evolutionary afternoon. Fossils record a prolonged series of changes. Some early mammaliaforms still retained connections between their middle-ear bones and the lower jaw. Complete separation occurred later and may have evolved independently in different mammalian groups.

Probainognathus stands near the beginning of this extraordinary anatomical story—not as the finished mammalian design, but as evidence that the old arrangement was already being altered.

A SMALL FOSSIL IN A VERY LARGE STORY

The Probainognathus fossil displayed at the Natural History Museum Abu Dhabi helps place mammals within the wider history of life. The museum’s exhibits carry visitors through billions of years of planetary change, and this unassuming cynodont earns its place among the giants.

Dinosaurs often dominate our vision of the Triassic and Jurassic worlds. They were large, spectacular and considerate enough to leave bones that look excellent in an atrium. Yet while dinosaurs were beginning their long reign, small cynodonts were undergoing an anatomical transformation that would ultimately produce the mammals.

Somewhere among their branches arose the earliest mammaliaforms. Their descendants survived the end-Triassic extinction, lived alongside the dinosaurs, endured the end-Cretaceous catastrophe and eventually diversified into nearly every terrestrial and marine environment on Earth.

The remarkable thing about Probainognathus is not that it was “almost us.” Evolution does not work toward a predetermined destination, and the creature certainly did not know that we would someday inspect its jaw for clues to the origin of the human ear.

It was simply a small predator trying to survive in Triassic Argentina.

But within its skull, old bones and new relationships had begun to overlap. A lower jaw built from several bones was moving toward one dominated by the dentary. An ancestral jaw joint was being joined by new contacts. 

Bones that still helped support feeding were entering an evolutionary process that would eventually place their descendants deep inside the mammalian middle ear.

The next time you chew while listening to someone speak, consider the two systems working on either side of your skull. One allows your dentary to move against the skull. The other uses three tiny bones to transmit the sound.

Their histories are intimately connected.

And part of that history can be seen in a modest little fossil in Abu Dhabi: Probainognathus, the progressive jaw that helped reveal how mammals learned to bite—and, eventually, to hear.

References and Further Reading

Romer, A. S. 1970. “The Chañares (Argentina) Triassic Reptile Fauna. VI. A Chiniquodontid Cynodont with an Incipient Squamosal-Dentary Jaw Articulation.” Breviora 344: 1–18.

Marsicano, C. A. et al. 2016. “The Precise Temporal Calibration of Dinosaur Origins.” Proceedings of the National Academy of Sciences 113: 509–513.

Martinelli, A. G., Soares, M. B. & Schwanke, C. 2016. “Two New Cynodonts from the Middle–Early Late Triassic of Brazil and Comments on South American Probainognathians.” PLOS ONE 11: e0162945.

Anthwal, N., Joshi, L. & Tucker, A. S. 2013. “Evolution of the Mammalian Middle Ear and Jaw: Adaptations and Novel Structures.” Journal of Anatomy 222: 147–160.

University of California Museum of Paleontology. Jaws to Ears in the Ancestors of Mammals.

Natural History Museum Abu Dhabi. Official Museum Website.

Lead Image: Asset id: 2757017209. Abu Dhabi UAE 8th Feb 2026: A Probainognathus fossil at the Natural History Museum Abu Dhabi reveals an early mammal-like cynodont, offering insight into the origins of mammals

Friday, 7 August 2026

AVES: LIVING DINOSAURS

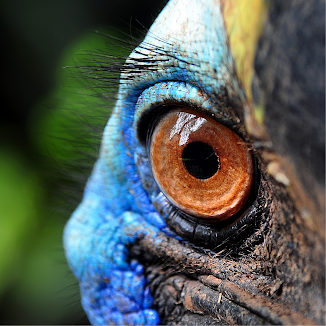
Cassowary, Casuariiformes
Wherever you are in the world, it is likely that you know your local birds. True, you may call them des Oiseaux, pássaros or uccelli — but you'll know their common names by heart.

You will also likely know their sounds. The tweets, chirps, hoots and caws of the species living in your backyard.

Birds come in all shapes and sizes and their brethren blanket the globe. It is amazing to think that they all sprang from the same lineage given the sheer variety. 

If you picture them, we have such a variety on the planet — parrots, finches, wee hummingbirds, long-legged waterbirds, waddling penguins and showy toucans. 

But whether they are a gull, hawk, cuckoo, hornbill, potoo or albatross, they are all cousins in the warm-blooded vertebrate class Aves. 

The defining features of the Aves are feathers, toothless beaked jaws, the laying of hard-shelled eggs, a high metabolic rate, a four-chambered heart, and a strong yet lightweight skeleton. The best features, their ability to dance, bounce and sing, are not listed, but it is how I see them in the world.

These modern dinosaurs live worldwide and range in size from the 5 cm (2 in) bee hummingbird to the 2.75 m (9 ft) ostrich. 

There are about ten thousand living species, more than half of which are passerine, or "perching" birds. Birds have wings whose development varies according to species; the only known groups without wings are the extinct moa and elephant birds.

Wings evolved from forelimbs giving birds the ability to fly
Wings, which evolved from forelimbs, gave birds the ability to fly, although further evolution has led to the loss of flight in some birds, including ratites, penguins, and diverse endemic island species. 

The digestive and respiratory systems of birds are also uniquely adapted for flight. Some bird species of aquatic environments, particularly seabirds and some waterbirds, have further evolved for swimming.

Wee Feathered Theropod Dinosaurs

We now know from fossil and biological evidence that birds are a specialized subgroup of theropod dinosaurs, and more specifically, they are members of Maniraptora, a group of theropods that includes dromaeosaurs and oviraptorids, amongst others. As palaeontologists discover more theropods closely related to birds, the previously clear distinction between non-birds and birds has become a bit muddy.

Recent discoveries in the Liaoning Province of northeast China, which include many small theropod feathered dinosaurs — and some excellent arty reproductions — contribute to this ambiguity. 

Still, other fossil specimens found here shed a light on the evolution of Aves. Confuciusornis sanctus, an Early Cretaceous bird from the Yixian and Jiufotang Formations of China is the oldest known bird to have a beak.

Like modern birds, Confuciusornis had a toothless beak, but close relatives of modern birds such as Hesperornis and Ichthyornis were toothed, telling us that the loss of teeth occurred convergently in Confuciusornis and living birds.

The consensus view in contemporary palaeontology is that the flying theropods, or avialans, are the closest relatives of the deinonychosaurs, which include dromaeosaurids and troodontids.

Together, these form a group called Paraves. Some basal members of this group, such as Microraptor, have features that may have enabled them to glide or fly. 

The most basal deinonychosaurs were wee little things. This raises the possibility that the ancestor of all paravians may have been arboreal, have been able to glide, or both. Unlike Archaeopteryx and the non-avialan feathered dinosaurs, who primarily ate meat, tummy contents from recent avialan studies suggest that the first avialans were omnivores. Even more intriguing...

Avialae, which translates to bird wings, are a clade of flying dinosaurs containing the only living dinosaurs, the birds. It is usually defined as all theropod dinosaurs more closely related to modern birds — Aves — than to deinonychosaurs, though alternative definitions are occasionally bantered back and forth.

The Earliest Avialan: Archaeopteryx lithographica

Archaeopteryx, bird-like dinosaur from the Late Jurassic
Archaeopteryx lithographica, from the late Jurassic Period Solnhofen Formation of Germany, is the earliest known avialan that may have had the capability of powered flight. 

However, several older avialans are known from the Late Jurassic Tiaojishan Formation of China, dating to about 160 million years ago.

The Late Jurassic Archaeopteryx is well-known as one of the first transitional fossils to be found, and it provided support for the theory of evolution in the late 19th century. 

Archaeopteryx was the first fossil to clearly display both traditional reptilian characteristics — teeth, clawed fingers, and a long, lizard-like tail—as well as wings with flight feathers similar to those of modern birds. It is not considered a direct ancestor of birds, though it is possibly closely related to the true ancestor.

Unlikely yet true, the closest living relatives of birds are the crocodilians. Birds are descendants of the primitive avialans — whose members include Archaeopteryx — which first appeared about 160 million years ago in China.

DNA evidence tells us that modern birds — Neornithes — evolved in the Middle to Late Cretaceous, and diversified dramatically around the time of the Cretaceous–Paleogene extinction event 66 mya, which killed off the pterosaurs and all non-avian dinosaurs.

In birds, the brain, especially the telencephalon, is remarkably developed, both in relative volume and complexity. Unlike most early‐branching sauropsids, the adults of birds and other archosaurs have a well‐ossified neurocranium. In contrast to most of their reptilian relatives, but similar to what we see in mammals, bird brains fit closely to the endocranial cavity so that major external features are reflected in the endocasts. What you see on the inside is what you see on the outside.

This makes birds an excellent group for palaeoneurological investigations. The first observation of the brain in a long‐extinct bird was made in the first quarter of the 19th century. However, it was not until the 2000s and the application of modern imaging technologies that avian palaeoneurology really took off.

Understanding how the mode of life is reflected in the external morphology of the brains of birds is but one of several future directions in which avian palaeoneurological research may extend.

Although the number of fossil specimens suitable for palaeoneurological explorations is considerably smaller in birds than in mammals and will very likely remain so, the coming years will certainly witness a momentous strengthening of this rapidly growing field of research at the overlap between ornithology, palaeontology, evolutionary biology and the neurosciences.

Reference: Cau, Andrea; Brougham, Tom; Naish, Darren (2015). "The phylogenetic affinities of the bizarre Late Cretaceous Romanian theropod Balaur bondoc (Dinosauria, Maniraptora): Dromaeosaurid or flightless bird?". PeerJ. 3: e1032. doi:10.7717/peerj.1032. PMC 4476167. PMID 26157616.

Reference: Ivanov, M., Hrdlickova, S. & Gregorova, R. (2001) The Complete Encyclopedia of Fossils. Rebo Publishers, Netherlands. p. 312.

Monday, 13 July 2026

DINOSAUR RIVALRY: MANTELLISAURUS

Mantellisaurus atherfieldensis 
This story begins some 125 million years ago on the lush floodplains of what is now the Isle of Wight, back in the Cretaceous.

Forget the cool, windswept English coastline of today. This was a warm, subtropical world of broad rivers, oxbow lakes and sprawling wetlands, where towering conifers, cycads and tree ferns sheltered one of Europe's richest dinosaur ecosystems. 

Early flowering plants were just beginning to appear, while insects buzzed through the forests and reptiles called across the floodplains.

Here, herds of Mantellisaurus atherfieldensis browsed on tender vegetation. At seven to eight metres (23–26 feet) long, these elegant herbivores were among the largest animals in their world. 

Their long hind limbs suggest they could move surprisingly quickly when needed—particularly if a hungry Neovenator emerged from the trees. 

Nothing encourages cardio quite like becoming someone else's lunch.

Its hands were every bit as remarkable as the rest of the animal. Projecting from each was a formidable thumb spike. Victorian artists loved depicting these dinosaurs charging into battle like armoured knights, but the reality was likely less theatrical. 

The spikes probably served as defensive weapons, may have helped settle disputes during the breeding season and perhaps even assisted in pulling down stubborn vegetation. Evolution has always appreciated a multitool.

The elongated fifth finger tells another story. Unlike the stout thumb, it was surprisingly flexible, capable of curling around branches to draw foliage closer—a wonderfully delicate adaptation for an animal weighing well over a tonne.

This specimen was discovered in 1914 by geologist Reginald Walter Hooley in the Upper Vectis Formation near Atherfield on the Isle of Wight. 

Described in 1917 and formally named Iguanodon atherfieldensis in 1925, it spent more than eighty years as a member of the ever-growing Iguanodon family.

That changed in 2007, when American palaeoartist and researcher Gregory S. Paul recognised that it was something quite different. 

More lightly built, with longer limbs and closer evolutionary ties to the African iguanodontian Ouranosaurus, it deserved a genus of its own. Paul named it Mantellisaurus, honouring Dr Gideon Algernon Mantell, the Sussex physician whose discoveries helped launch the science of dinosaurs.

Mantell's story is one of brilliance, perseverance and one of Victorian science's greatest rivalries.

In 1822, he described Iguanodon, only the second dinosaur ever scientifically named.

Mantell spent decades collecting fossils and championing these extraordinary animals, only to find himself increasingly at odds with the formidable anatomist Sir Richard Owen.

Owen coined the word Dinosauria and later became the driving force behind London's Natural History Museum, but he also had a habit of eclipsing rivals—and few felt that more keenly than Mantell. The two men disagreed about almost everything, from dinosaur anatomy to broader questions of evolution, as they emerged in Victorian science.

Mantell increasingly recognised that these animals were active, lightly built and far more dynamic than giant lizards. Owen preferred to reconstruct them as slow, heavily built, rhinoceros-like reptiles that fit comfortably within his creationist view of nature.

When Benjamin Waterhouse Hawkins created the famous Crystal Palace dinosaurs during the 1850s, it was Owen's interpretation that guided the sculptures. 

Visitors marvelled at enormous reptilian beasts, including an Iguanodon sporting what appeared to be a horn proudly perched upon its nose.

As science advanced—and as more complete skeletons were discovered, particularly the spectacular Bernissart specimens from Belgium—we learned that the famous "horn" was, in fact, the thumb spike.

One of the most iconic mistakes in palaeontology had become one of its best-known corrections.

Tuesday, 7 July 2026

FEATHERED SHOW-OFF OF THE CRETACEOUS: OVIRAPTOR

If ever there were a dinosaur that looked like it had dressed for a gala while everyone else showed up in sensible hiking boots, it was Oviraptor.

Picture yourself standing on the warm floodplains of Mongolia some 75 million years ago. The air shimmers with heat. 

Ferns rustle gently in the breeze. Somewhere nearby, insects hum while distant hadrosaurs grumble to one another. 

Then, stepping lightly between low shrubs, comes a creature unlike almost any other dinosaur.

About the size of a large turkey—though with considerably better posture—Oviraptor carries itself with quiet confidence. 

Its toothless beak gleams in the sunlight, its elegant neck curves gracefully, and atop its head rises a tall, bony crest that seems almost purpose-built for showing off. 

Draped across its body are feathers that catch the light with flashes of bronze, emerald, copper and midnight blue, colours that shift with every movement. 

Much like the iridescent plumage of today's magpies, starlings and peacocks, those shimmering feathers may have dazzled rivals and potential mates alike.

It is difficult not to smile looking at this wonderful oddball. Despite its fearsome name—Oviraptor means "egg thief"—it has spent more than a century trying to clear its reputation.

The first Oviraptor fossils were discovered in 1923 during the American Museum of Natural History's legendary Central Asiatic Expeditions to the Gobi Desert of Mongolia, led by the adventurous Roy Chapman Andrews. 

At the spectacular fossil beds of Bayn Dzak—the famous Flaming Cliffs—the expedition uncovered a partial skeleton lying beside a clutch of fossil eggs. It was a sensational find.

Henry Fairfield Osborn formally described the animal in 1924, naming it Oviraptor philoceratops—"egg thief, lover of ceratopsian eggs." 

We believed for many years that the dinosaur had been caught red-handed, stealing the eggs of Protoceratops. It made for a wonderfully dramatic story.

There was just one small problem. The story was wrong.

Decades later, beautifully preserved embryos discovered inside similar eggs revealed that they belonged not to Protoceratops, but to Oviraptor and its close relatives. 

Even more extraordinary were fossils of adults preserved sitting over their nests with their feathered forelimbs spread protectively around their eggs, as many modern birds do today. 

Rather than a notorious nest robber, Oviraptor appears to have been an exceptionally devoted parent that likely died defending its own young during a sudden sandstorm. While this all played out millions of years ago, it still pulls at my heartstrings. 

Talk about a public relations disaster. If dinosaurs had lawyers, Oviraptor would almost certainly have won its defamation case.

Those remarkable fossils revealed something else just as exciting. Adults carefully brooded their nests with feathered arms extended over the eggs, insulating them while allowing air to circulate. It is a strategy remarkably similar to that used by many birds today and a beautiful reminder that some of the most familiar behaviours in our backyards have roots deep in the Age of Dinosaurs.

Oviraptor belonged to a remarkable group of feathered theropods called oviraptorosaurs. These animals shared a common ancestor with the lineage that ultimately gave rise to modern birds. While Oviraptor itself was not a direct ancestor of living birds, it sits close to that evolutionary branch, preserving many features we now think of as unmistakably avian.

Its lightweight skeleton, hollow bones, wishbone (furcula), feathers, bird-like wrists and remarkable nesting behaviour all tell the story of dinosaurs becoming birds—not in one dramatic leap, but through millions upon millions of years of evolutionary refinement.

Its beak was another clever adaptation. Rather than relying on rows of sharp teeth, Oviraptor likely used its powerful jaws to crack open nuts, seeds, shellfish and other tough foods. It probably sampled the occasional egg when opportunity presented itself—as plenty of modern birds do—but certainly not often enough to deserve becoming prehistory's most infamous "egg thief."

And that magnificent crest? It was almost certainly less about battle than beauty.

Think of it as the Late Cretaceous equivalent of an extravagant hairstyle. Like the casque of a cassowary or the elaborate adornments of hornbills, the crest probably helped attract mates, establish dominance and identify individuals. Nature, it seems, has always had a flair for dramatic fashion.

Many of the behaviours we delight in watching among birds today—displaying, nesting, brooding, caring for young—were already well established while Tyrannosaurus still ruled the landscape.

Every new feathered dinosaur we uncover paints a picture of the Late Cretaceous as a landscape alive with colour, courtship displays, parental devotion and astonishing diversity. 

Flashing feathers shimmered in the sunlight. Elaborate dances played out across ancient floodplains. Tender parents guarded carefully tended nests while giant predators stalked the horizon.

Their descendants bring me joy each morning as I enjoy my first coffee of the day listening to their hoots and calls. The dinosaurs never truly disappeared. Some simply traded thunderous footsteps for morning birdsong.

Fossil Oviraptor Image: Danny Ye, License: 2765957049

Monday, 22 June 2026

LURKING IN THE LATE CRETACEOUS: RAJASAURUS

Rajasaurus narmadensis
In the humid, fern-thick forests of Late Cretaceous India — about 67 million years ago — a flash of red moves between the tree trunks.

Think oxidized iron and dried blood — deep crimson-orange broken by pale white striping and bold black bands along the flanks and tail. 

In dappled forest light, those stripes would fracture the animal’s outline, a trick modern tigers use to unnerving effect. Camouflage is not new. Evolution figured that out long before mammals started prowling.

This is Rajasaurus narmadensis, the “king lizard of the Narmada,” known from the Lameta Formation of central India. 

At roughly 6–7 meters long and weighing perhaps a metric ton, it was not the largest theropod of its time — but it did not need to be. It was built for hunting.

Rajasaurus belongs to the Abelisauridae, a clade of short-snouted, deep-skulled theropods that dominated the southern continents of Gondwana. If you squint, you can see its relatives in Madagascar’s Majungasaurus, Argentina’s Carnotaurus, and Africa’s Rugops. These animals were the southern answer to the tyrannosaurs of the north.

Unlike the long-snouted, banana-toothed elegance of Tyrannosaurus rex, abelisaurids had blunt, boxy skulls and often elaborate cranial ornamentation. Rajasaurus sported a single low horn or dome on its forehead — not a unicorn spike, but a thickened bony crest. 

It likely served for display, species recognition, or perhaps ritualized head-shoving contests. Theropods were dramatic. This is not speculation; this is pattern recognition across deep time.

Its forelimbs? Tiny. Comically so. Abelisaurids doubled down on arm reduction — evolution looked at the T. rex blueprint and said, “Let’s go smaller.” The arms were functionally irrelevant in prey capture. This was a head-driven predator. And what a head it was.

Rajasaurus lived in interesting times. Late Cretaceous India was not yet welded to Asia. It was a drifting island continent, sliding northward across the Tethys Ocean. The climate was warm, seasonally dry, punctuated by monsoonal rains. River systems braided across floodplains. Forests of conifers, palms, and flowering plants thickened along waterways. Ferns and horsetails crowded the understory.

Sharing that forest were enormous titanosaurian sauropods, including forms like Isisaurus and Jainosaurus. Long-necked, barrel-bodied giants moved in herds, stripping vegetation and reshaping the landscape as they fed. Their hatchlings and juveniles would have been very much on Rajasaurus’s radar.

Small ornithischian dinosaurs darted through the brush. Crocodyliforms basked along muddy riverbanks. Turtles paddled in oxbow lakes. Mammals — small, mostly nocturnal insectivores — kept wisely out of sight.

Pterosaurs likely wheeled overhead. Insects buzzed. The forest was noisy, layered, alive.

And somewhere within it, Rajasaurus was listening.

Abelisaurids had thick necks and reinforced skulls. Biomechanical studies of relatives like Majungasaurus suggest a predatory style focused less on bone-crushing bite force and more on repeated, slashing bites combined with powerful neck musculature. Think controlled violence rather than single catastrophic impact.

Rajasaurus likely relied on ambush. In dense forest cover, speed over short distances would matter more than marathon endurance. Its hind limbs were strong and proportioned for bursts of acceleration.

Picture it waiting — body low, tail held rigid for balance. A subadult titanosaur lingers near the herd’s edge. A misstep. A moment of distraction. The red-and-white predator explodes from cover.

The jaws close around soft tissue — flank, neck, perhaps hind limb — and then release. Another strike. And another. Blood loss and shock do the rest. Abelisaurids may not have grappled like dromaeosaurs or crushed like tyrannosaurs, but they were efficient.

And they were persistent.

There is even evidence of cannibalism among some abelisaurids (looking at you, Majungasaurus), so it’s not unreasonable to suspect Rajasaurus would not waste protein when opportunity presented itself. 

The predators of the Late Cretaceous were not sentimental.

Phylogenetically, Rajasaurus sits within Abelisaurinae, closely related to Majungasaurus of Madagascar and South American forms such as Carnotaurus sastrei. This distribution tells a broader tectonic story — these predators evolved across the southern fragments of Gondwana before continental breakup isolated their lineages.

India’s northward drift preserved a snapshot of this southern evolutionary experiment just before the asteroid impact that would end the non-avian dinosaurs.

Rajasaurus lived within a few million years of that event. Which means this red-striped hunter walked forests that would soon vanish under global firestorms, impact winter, and ecological collapse.

The gorgeous illustration you see here is by the supremely talented Daniel Eskridge, licensed for use. Appreciate you, Daniel. 


Timing, as ever, is everything.